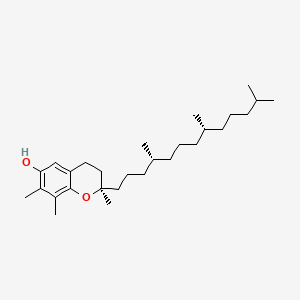
Why these belong in the same formula. Each row says what the basis is, from settled biochemistry through to a trial that measured the pair.
Supplemental alpha-tocopherol is preferentially retained by hepatic alpha-tocopherol transfer protein and lowers serum and tissue gamma-tocopherol. A vitamin E product built only on alpha therefore reduces the isoform this ingredient supplies.
The tocopherol isoforms share absorption, lipoprotein loading and the same transfer protein, which favours alpha and clears gamma faster. Mixed tocopherol blends exist because a high alpha dose crowds out gamma.
Tocopherols and tocotrienols compete for the same absorption and transport machinery, and a high alpha-tocopherol content interferes with tocotrienol retention most of all. Full-spectrum products keep gamma and the tocotrienols together with alpha kept low.
After a tocopherol quenches a lipid radical it becomes a tocopheroxyl radical, which ascorbate at the membrane surface reduces back to the active form. The pairing recycles the tocopherol rather than consuming it once.
Tocopherols intercept lipid peroxyl radicals in the membrane while selenium-dependent glutathione peroxidase removes the peroxides that form. The two defences are complementary and were characterised together.
Ubiquinol sits in the same lipid bilayer and can reduce the tocopheroxyl radical back to tocopherol. That regeneration keeps the tocopherol pool active during sustained oxidative load.
Glutathione restores ascorbate, which in turn restores the tocopheroxyl radical, so the tocopherol pool depends on the thiol pool upstream. The three form a described relay across the aqueous and lipid phases.
Dihydrolipoic acid regenerates ascorbate and glutathione, which in turn regenerate the tocopheroxyl radical. Its dual water and lipid solubility lets it feed both sides of that relay.
Long-chain polyunsaturated fatty acids oxidise readily, and tocopherols are added to fish oils to intercept the chain reaction. Taking them together also gives the fat-soluble tocopherol the lipid vehicle it needs for absorption.
EPA and DHA carry many double bonds and are the most peroxidation-prone fats in a formula, which tocopherols are used to stabilise in the capsule and in the membrane. The oil also acts as the carrier that raises tocopherol absorption.
Tocopherols are absorbed in mixed micelles and their uptake is poor from a fat-free dose, so a lipid carrier raises delivery. Medium-chain triglycerides are used for that purpose and are not themselves peroxidation-prone.
Tocopherols and carotenoids share micellar solubilisation and lipoprotein transport, so large doses of one can lower the uptake of the other in the same meal. Splitting fat-soluble actives across doses reduces that crowding.
Large tocopherol doses have been reported to interfere with vitamin K-dependent carboxylation, an effect documented mainly for high-dose alpha-tocopherol. Formulas keeping both should hold tocopherol amounts moderate.
When gamma-tocopherol quenches a lipid radical it becomes a tocopheroxyl radical that must be reduced back to the active phenol. Ascorbate and glutathione do that reduction, and glutathione is returned to its reduced state by glutathione reductase, an FAD enzyme built from riboflavin. Riboflavin status therefore sits upstream of how quickly any tocopherol pool is recycled. This is settled biochemistry rather than a combination trial.
Gamma-Tocopherol + NACEstablished precursor relationship: N-acetylcysteine supplies cysteine for glutathione synthesis, and glutathione participates in tocopherol radical recycling. Cysteine availability is the rate-limiting step in glutathione synthesis. A larger reduced glutathione pool supports faster return of tocopheroxyl radicals to the phenol form inside membranes. The relationship is a chain of established reactions, not a measured clinical outcome.
Free cysteine feeds gamma-glutamylcysteine synthetase, the committed step of glutathione synthesis. Glutathione then supports the ascorbate and thiol network that keeps membrane tocopherols in their reduced form. No combination trial is implied here, only the shared pathway.
Glutathione is glutamate, cysteine and glycine. Low glycine availability constrains the final ligase step and therefore the size of the reduced glutathione pool that supports tocopherol recycling. The connection is stoichiometric biochemistry.
Gamma-Tocopherol + LycopeneEstablished shared chemistry: both are lipid-phase antioxidants carried in the same lipoprotein compartment, and carotenoids and tocopherols compete for micellar space. Lycopene and gamma-tocopherol both need dietary fat, bile and mixed micelles to cross the enterocyte, and they travel together in chylomicrons and LDL. Large single doses of one lipid-soluble antioxidant can crowd micellar capacity for another. In the membrane phase their radical-scavenging chemistry is complementary rather than identical, since lycopene handles singlet oxygen and tocopherols chain-break lipid peroxidation.
Lutein and tocopherols are solubilised in the same mixed micelles and taken up partly through the same enterocyte transporters. Taken together in large amounts they can reduce each other's uptake from a single meal. Spacing or splitting across meals is the ordinary formulation response.
Quercetin partitions at the lipid and water interface where tocopheroxyl radicals sit, and phenolic hydrogen donation to that radical has been characterised in model lipid systems. Human data on the pair is thin, so this is a mechanism-level pairing rather than an outcome. Presented as chemistry, not as an effect a person would feel.
Proanthocyanidins act as hydrogen donors at the aqueous face of a membrane, the same place the tocopheroxyl radical presents its phenolic oxygen. That makes the two chemistries complementary in vitro. Human outcome data for the specific pair is limited, so the confidence stays mid.
Polyunsaturated fatty acid supplements raise the amount of oxidisable lipid carried in membranes and lipoproteins, which is why tocopherols are routinely formulated alongside them. A published supplementation study combined omega-3 and omega-6 fatty acids with antioxidant vitamins in the same protocol. The pairing is a formulation and lipid-chemistry rationale, not a demonstrated additive outcome.
Tocopherols are absorbed only after they enter mixed micelles built from bile salts, phospholipids and fatty acids. Added phospholipid raises the dispersibility of an oil-phase tocopherol in the gut lumen. This is why so many tocopherol softgels sit in a lecithin-containing oil base.
Lecithin is a mixed phospholipid emulsifier used to keep tocopherol in a fine dispersion in the capsule oil and in the gut. It contributes to micelle formation alongside bile. It is a carrier role rather than an independent active pairing.
Gamma-Tocopherol + RosemaryEstablished antioxidant formulation practice: rosemary extract and tocopherols are used together to slow oxidation of an oil phase. Carnosic acid and carnosol act as chain-breaking antioxidants in the same oil that carries tocopherols, and the two classes are commonly combined to protect the oil itself. That is about the stability of the product in its capsule. It says nothing about an effect inside the body.
Gamma-Tocopherol + ZincEstablished cofactor relationship: zinc is structural in copper-zinc superoxide dismutase, which sits upstream of lipid peroxidation. Superoxide dismutase converts superoxide to hydrogen peroxide before it can react further and start lipid chain reactions, while gamma-tocopherol acts inside the membrane once a chain has begun. The two work at different points of the same sequence. Complementary positions in one pathway, not a measured combination effect.
Gamma-Tocopherol + CopperEstablished cofactor relationship for copper-zinc superoxide dismutase, plus the pro-oxidant behaviour of free copper toward lipids. Bound copper is needed for superoxide dismutase activity. Unbound copper is a classic catalyst of lipid peroxidation in vitro, which is exactly the reaction chain a tocopherol interrupts. The direction depends entirely on whether the copper is protein-bound, and that nuance belongs on the row.
Mitochondrial membranes are lipid-rich and are where much superoxide originates. Manganese superoxide dismutase removes that superoxide, while membrane tocopherols stop propagation once peroxidation starts. Two different steps of one defence sequence.
Silymarin flavonolignans are hydrogen donors that partition into membranes and lipoproteins. In model systems phenolic donors of this class can regenerate a tocopheroxyl radical. Human evidence for the pair specifically is limited, so this stays at a mechanism-level claim.