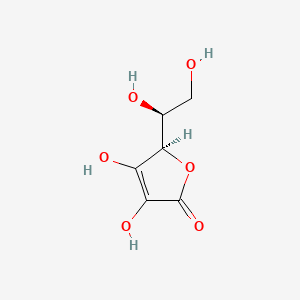
Why these belong in the same formula. Each row says what the basis is, from settled biochemistry through to a trial that measured the pair.
When vitamin E quenches a fat-soluble radical inside a membrane it is left as a spent radical itself, and vitamin C donates an electron to return it to the working form. Vitamin C works on the watery side and vitamin E within the membrane, so the two cover both compartments of one recycling loop.
After vitamin C gives up an electron it becomes dehydroascorbate, and glutathione is one of the main reductants that converts it back to the active vitamin. NAC supplies the cysteine that is rate-limiting for making glutathione, so it helps keep the pool that regenerates vitamin C replenished.
Lysine residues in procollagen are hydroxylated by an ascorbate-dependent enzyme before cross-links can form. The pairing of lysine with ascorbate follows from that single reaction.
Ascorbate and glutathione regenerate each other's oxidised forms, so each spares the other. The interplay is a textbook part of the cellular redox network.
Dihydrolipoate reduces dehydroascorbate back to ascorbate, returning the vitamin to its working form. The two sit in the same regeneration chain as glutathione and vitamin E.
Two of the four steps that build carnitine from trimethyllysine are ascorbate-dependent dioxygenases. Endogenous carnitine formation slows when ascorbate is short.
Ascorbate reduces the quercetin radical back to the parent flavonoid and quercetin in turn slows ascorbate oxidation, and the two also share cellular transport routes. They are conventionally formulated together for that reason.
Acerola delivers ascorbate together with the anthocyanins and organic acids that occur with it in fruit, so it contributes to the same vitamin C total. Amounts from both sources should be added, not counted separately.
Ascorbate reduces cupric to cuprous copper and large sustained doses can interfere with ceruloplasmin-bound copper, lowering measured copper status. Balanced amounts rather than very high ascorbate alone keep copper handling normal.
Ascorbate keeps reduced folates from oxidising in the formulation and in gastric contents. Co-formulation is standard for that stability reason.
With a plain ferrous salt, ascorbate keeps the iron reduced and raises the fraction absorbed. The same chemistry also keeps more free iron redox-active in the gut lumen, which is the mechanism behind the nausea and gastric complaints some people report on the pairing. Worth flagging both directions rather than only the uptake side.
A glycine chelate keeps iron bound through the gut, so it depends less on ascorbate to stay soluble than an ionic salt does. Co-dosing with vitamin C is common practice and is not expected to hurt, but the added benefit is smaller when the iron is already chelated. This is reasoning from the chelate chemistry, not from a head-to-head trial.
Prolyl hydroxylase converts proline residues in the procollagen chain to hydroxyproline, and it needs ascorbate to keep its iron centre reduced. Without that step the triple helix is unstable. Proline supplies the residue, ascorbate keeps the enzyme running, so the two sit on the same step from opposite sides.
Tyrosine feeds the catecholamine pathway, and the final step from dopamine to norepinephrine runs through dopamine beta-monooxygenase, a copper enzyme that uses ascorbate as its electron donor. Ascorbate is concentrated in secretory vesicles for exactly that job. This is settled biochemistry and not a claim that the pair changes mood or focus.
Ascorbic acid can degrade cobalamin in solution, which is why analytical and formulation work keeps large amounts of the two apart in liquids. Whether swallowing them together meaningfully lowers B12 status in a person is not settled. Formulators separate them in liquids and effervescents as a precaution rather than because a deficit has been demonstrated.
Carotenoids quench radicals inside the lipid phase while ascorbate works in water, and ascorbate can reduce carotenoid radical cations back to the parent molecule at the interface. The pairing is mechanistic rather than an outcome that has been measured as a clinical benefit. Both are commonly co-formulated for that reason.
Astaxanthin spans the membrane and takes radicals in the lipid layer. Ascorbate handles the aqueous side and can help return oxidised partners to their reduced form. The chemistry is well described in model systems. Human co-supplementation data specific to this pair is thin, so it belongs at low confidence.
EPA and DHA are highly oxidisable, and antioxidant coverage in the aqueous compartment limits the propagation step that follows a peroxyl radical forming. Ascorbate itself sits in water, so it works through the tocopherol it regenerates rather than inside the oil. Note the direction: it helps guard the fat, it does not add to the omega-3 effect itself.
Dietary nitrate becomes nitrite via oral bacteria, and in the acidic stomach ascorbate speeds the non-enzymatic conversion of nitrite to nitric oxide. That chemistry is well characterised. Whether adding vitamin C to a nitrate dose changes a performance or vascular readout in people has not been settled here.
Nitric oxide synthase needs tetrahydrobiopterin as a cofactor, and ascorbate slows the oxidation of that cofactor so the enzyme stays coupled to arginine rather than producing superoxide. Arginine is the substrate, ascorbate protects the cofactor. This describes the pathway, not a measured vascular outcome for the combination.
EGCG oxidises readily at neutral pH, and ascorbate in the same drink or capsule slows that loss, which is why bottled green tea products carry ascorbate. More intact catechin reaching the intestine is the plausible route to higher exposure. The evidence sits at the chemistry and pharmacokinetic level rather than at a clinical endpoint.
Proanthocyanidins are effective one-electron donors and ascorbate can regenerate some phenolic radicals back to their reduced form, so the two overlap in the same aqueous compartment. The pairing is long-standing in formulation practice. It is mechanistic reasoning at low confidence, not a demonstrated additive effect in people.
Selenium is built into glutathione peroxidase, which clears peroxides using glutathione. Ascorbate helps keep glutathione in its reduced form. The two support normal antioxidant handling from different points in the same system. Co-supplementation is routine, and the connection is mechanistic rather than an outcome measured for the pair.
Calcium ascorbate is a buffered salt used when plain ascorbic acid feels harsh, so the calcium here is part of the delivery rather than a separate active. Anyone counting total calcium intake should include what the ascorbate salt contributes. The buffering changes the pH of the dose, not the vitamin activity.
Zinc and vitamin C appear together in immune-support formulas more often than almost any other pair, each with its own role in normal immune function. No absorption interaction of consequence is described between them at ordinary doses. The pairing is formulation convention plus two separate nutrient roles, not a demonstrated interaction.
Non-heme iron, the kind in plants and most supplements, is absorbed as ferrous iron, and vitamin C keeps it in that reduced form and binds it into a soluble complex in the stomach. Taken in the same dose, vitamin C raises how much of the iron the gut takes up and blunts the inhibiting effect of the phytates and polyphenols in a meal.
The body builds collagen by hydroxylating proline and lysine on the new chain, and the enzymes that do it need vitamin C as a cofactor. Without it the chains cannot fold into a stable triple helix. Collagen peptides supply the amino acids. Vitamin C lets the cell assemble them.